Main
In coastal regions characterized by high flood risk, people and assets are commonly protected from flooding by dikes, dams and sea walls; so-called grey flood protection. These engineered structures are increasingly challenged by changes in local and regional climate conditions, such as sea level rise, land subsidence and increased storm exposure, and may become unsustainable1. Hard engineering structures are static and do not adapt to a changing environment2. Therefore, so-called green–grey flood protection—which combines traditional grey-protection with green-ecosystems—is increasingly considered a more sustainable strategy for keeping coastal regions safe from storm events with extreme waves3.
Green–grey flood protection uses the natural capacity of ecosystems to buffer extreme wave events and consequently reduce flood risk. Specifically, salt marshes with unique salt-tolerant vegetation4, often located in the temperate climate zone at muddy coasts, serve to attenuate large waves during storm surge events5.
Salt marshes attenuate waves by dissipating wave energy due to (1) the elevated bed6, and (2) the drag and roughness of the vegetation growing in the marsh7,8,9,10,11. Both are expected to change during extreme wave events, thereby decreasing the wave-attenuating capacity. Studies so far have indicated that marsh substrates remain stable under moderate storms (significant wave height under 1 m), whereas stability under extreme wave exposure (wave height exceeding 1 m) has not been tested. At the same time, above-ground vegetation breaks and detaches from the marsh surface during moderate storms5,12. Modelling studies extrapolating field evidence highlight that nearly all vegetation is broken after exposure to waves up to 1 m (ref. 13), inevitably leading to decreasing wave attenuation5,13,14. Overall, there seems to be a relationship between wave forcing and vegetation loss: as a storm lasts longer, above-ground vegetation is progressively damaged and wave attenuation diminishes.
In several regions, future storm surges are expected to exceed the water levels that have been assessed in laboratories so far (maximum of 2 m)5,15 ; for example, the UK16 and the Netherlands15. Such surges are also predicted to occur with a 25-year return period in the Yellow Sea and East China Sea (China); the Gulf of Carpentaria (Australia); the Bay of Bengal (Bangladesh); and the Gulf and East coast of the United States17. Surge levels are expected to increase even further in the coming decades18. There is a lack of quantified knowledge explaining progressive vegetation damage and potential substrate erosion under these conditions, and the efficacy of damaged marsh vegetation in wave attenuation during extreme wave events (>1 m).
Based on flume experiments and projected storm simulations at a global scale, here we aim to quantify the persistence of the marsh substrate and address the progressive vegetation damage and associated reduced wave attenuation under extreme storm conditions, by assessing:
-
I.
The stability of salt marsh substrate under extreme wave events.
-
II.
Progressive vegetation damage and associated wave attenuation under extreme events.
-
III.
The global contribution of progressively damaged salt marsh vegetation to wave attenuation that proceeds from results of the flume experiments.
Natural marsh in a large-scale flume
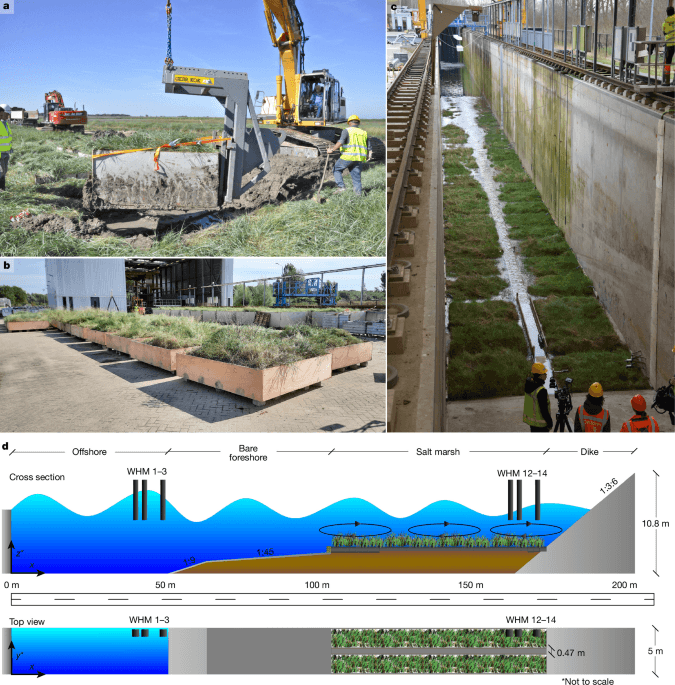
A 306-m2 salt marsh with intact above-ground biomass and marsh substrate was installed in the Delta Flume, a 300-m-long, 5-m-wide and 9.5-m-high wave flume (Deltares, Delft, the Netherlands), enabling a full-scale test. A winter-state salt marsh was transplanted to two cross-shore transects using the first 200 m of the flume (Fig. 1). The marsh, fronting the dike, was characterized by a high density of marsh vegetation species, dominated by Elymus athericus (E. athericus), but with Atriplex prostrata present at lower densities (Methods). Such vegetation is present at a high elevation in the tidal regime, which makes it effective in attenuating waves14,15.
a, Obtaining the salt marsh blocks in the field at the Dutch mainland Wadden Sea coast. b, Storing the blocks next to the Delta Flume at Deltares. c, Inundating the full physical model. d, A schematic of the physical model with the salt marsh blocks from the field in the Delta Flume, with the wave paddle at X = 0 m and locations of the wave height meters (WHMs) indicated. Visualizations of wave forcing, as well as attenuation through vegetation drag and roughness, are shown.
Extreme conditions were simulated over the marsh (Fig. 1). The water depth above the salt marsh surface ranged between 1.5 m and 4 m, and the hydrodynamic conditions reproduced depth-limited waves, with maximum significant wave heights (Hm0) set to half of the local water depth. Offshore significant wave heights ranged between 0.75 m and 2 m. The marsh was exposed for a total duration of approximately 29 h, of which 21 h included above-ground vegetation, whereas the last 8 h occurred without above-ground vegetation, but with largely intact below-ground biomass (see Methods and Supplementary Table 1 for the testing programme). The lower end of this range is equal to field observations and past flume experiments, with wave heights of 0.85 m (ref. 12) and 0.90 m (ref. 5). The upper end of the range represents extreme events, for example, in the Western Scheldt (the Netherlands) and Chesapeake Bay (United States)14,19.
Marsh substrate under extreme storms
Whether salt marshes effectively contribute to wave attenuation primarily depends on the stability of the marsh substrate. When the substrate erodes, below- and above-ground vegetation biomass might also be (partly) removed. Elevation measurements at 32 fixed locations at the salt marsh show, on average, a decreasing marsh surface over the total experimental time of 21 h with damaged vegetation (7 mm; 0.33 mm h–1), which is in the same order of magnitude as previous studies with smaller wave heights (4.4 mm surface lowering; 0.16 mm h–1)5,20, and smaller-than-typical length scales of the marsh microtopography (Methods). The presence of below-ground biomass and roots in the marsh substrate is known to enhance soil stability. A clear root zone was also present in our experiment, mainly in the top 10 cm of the substrate. The observed stable marsh platform aligns with past observations of hurricanes (Katrina and Rita) that eroded 527 km2 of mainly brackish marshes in the Louisiana coastal plain. Salt marshes remained stable and largely unchanged21. The stability of the marsh substrate under extreme conditions is an essential feature for marsh existence in areas in which regular wave attacks may be expected22. Our experiment shows that this essential feature is also valid for extreme storms, which agrees with past field and flume evidence20,21,23. Thus, with negligible surface erosion and largely intact below-ground vegetation biomass throughout all experimental runs, our experiment suggests that marsh platforms are able to contribute to wave attenuation irrespective of the short-term damage to above-ground biomass, as long as there is no lateral retreat due to seaward cliff initiation and erosion24,25. We therefore focus hereafter on progressive vegetation damage reducing wave attenuation over time.
Wave attenuation and vegetation damage
Salt marsh vegetation breaks under prolonged wave exposure5,13,26. Consequently, the above-ground biomass that contributes to wave attenuation decreases. The experimental runs are clustered into three distinct groups of repeating wave height and water depth combinations. In the first two groups, continuous wave exposure caused progressively increasing damage to the above-ground vegetation, whereas the above-ground vegetation was removed in the last group (Methods and Supplementary Table 1). This allowed us to explicitly quantify wave attenuation by vegetation as a result of progressive damage of the above-ground biomass.
The above-ground biomass present in the flume before the experiment started did not statistically differ from the vegetation found in the field during the same period (Mann–Whitney U test; P > 0.05) (Fig. 2). Initially, after the first experimental run, above-ground biomass and vegetation stem length largely decreased by 33% (from 831 g m–2 to 558 g m–2) and 19% (from 56 cm to 45 cm), respectively (Fig. 3a,b). Although vegetation damage increased with exposure duration, the above-ground biomass and stem length did not change significantly across the experimental runs with different wave forcing, apart from biomass during the last experimental run with a significant wave height of 2 m (t-test for normal and Mann–Whitney U test for not normal distributed samples; Benjamini–Hochberg FDR P-value correction; P > 0.05; Supplementary Table 2). Throughout the experimental runs, visual inspection showed that vegetation damage was greatest close to the seaward vegetation edge. Above-ground biomass changed significantly after approximately 21 h of wave exposure (Welch t-test; Benjamini–Hochberg FDR P-value correction; P < 0.01) and decreased to 20−25% of the initial biomass, while stem length decreased significantly over time by 47%, with an average height of 0.29 m remaining over the full marsh (Fig. 3b) (Welch t-test; Benjamini–Hochberg FDR P-value correction; P < 0.01).
Dry biomass (mean and standard error) in the field (field T0), in the flume before (flume T0) and after (Tend) the experimental runs with above-ground vegetation.
a,b, Dry biomass (a) and stem length (b) decrease over exposure duration, with median (horizontal blue lines) and mean (horizontal dashed black lines). c, The contribution of above-ground vegetation stem length to wave attenuation for different tested significant wave heights (Hm0 = 0.75 m, 1.25 m, 2 m) and the linear fits for the tested wave heights. d, Exposure duration related to wave height attenuation by vegetation in a generalized linear model (GLM) and a verification of the model (inset).
The above-ground vegetation consistently contributed to wave attenuation over the salt marsh platform, despite the progressive damage (Fig. 3c). The largest attenuation was observed for the smallest waves of Hm0 = 0.75 m (between 6% and 22%), whereas vegetation contributed the least to attenuation for the largest waves of Hm0 = 2 m (between 0% and 6%)15. Moreover, the effect of vegetation damage on the decreasing contribution of vegetation to wave attenuation was more pronounced for smaller than for larger waves. The experimental results emphasize a potentially large contribution to wave attenuation for incoming wave heights at the lower range of the experimental program (below 1 m).
The experimental results are described by a generalized linear model (GLM), which uses exposure duration and incoming wave height as predictors and wave attenuation by vegetation as response variable (pseudo R2 = 0.97; measured versus predicted R2 = 0.93; Methods). Following past studies during high waves, vegetation damage starts at significant wave heights of approximately 0.5 m (refs. 5,27) and continues with the increasing heights observed in our experiment. Vegetation damage also increases with exposure duration.
Global contribution of marsh vegetation
To analyse the contribution of vegetation to wave attenuation under extreme wave conditions, extending the experimental results to the global scale, we use global datasets for storm surge hydrographs28; coastal elevation data along coast-normal transects29, which are updated using DeltaDTM30; and recent salt marsh presence maps31, which are combined with the GLM (Methods). Exposure duration, vegetation stem height damage and subsequent wave attenuation by vegetation were calculated at the storm surge peak for storms, with a return period of 100 and 1,000 years (Methods). The vegetation biomass and stem height of E. athericus applied in our experiments are in the lower range for salt-marsh-vegetation-carrying stems (Methods and Extended Data Fig. 1) and can be considered a conservative estimator for wave attenuation by salt-marsh-vegetation-carrying stems29,32,33.
The global analysis shows that approximately half of the marshes are exposed for 200 to 400 min during a single storm, emphasizing a small window for progressive vegetation damage and decreasing wave attenuation capacity (Fig. 4a; Extended Data Fig. 2a; Supplementary Figs. 1 and 2). The longest observed exposure duration was 1,000 min for both return periods, resulting in maximum 50% vegetation damage (Fig. 4b and Extended Data Fig. 2b). Wave attenuation calculations using the GLM resulting from the flume experiment highlight a clear distinction (Fig. 4c and Extended Data Fig. 2c): waves are effectively attenuated at lower energy salt marsh coasts with incoming waves up to 1 m. At these low-energy marsh coasts, wave attenuation by vegetation generally exceeds 10% (up to 50%), covering up to half of the analysed transects (46−34%, for return periods of 100 and 1,000 years, respectively). By contrast, wave attenuation is limited to only 10% at high-energy marsh coasts where incoming wave heights exceed 1 m.
a, Exposure duration (min) for progressive vegetation damage and distribution for a return period of 100 years. b, Relative stem height decrease and distribution (%) for a return period of 100 years. c, GLM-predicted attenuation by vegetation (%) and distribution per wave attenuation, and incoming wave height bin for a return period of 100 years.
Marsh vegetation reducing extremes
The experimental results in this study contribute to understanding salt marsh–wave interactions under extreme events: vegetation is progressively damaged and wave attenuation decreases, while the bed remains stable. Projecting results from the flume experiments to a global scale suggests that salt marsh vegetation generally enhances the resistance of low-energy marsh coasts to extreme conditions. Results emphasize that at almost all low-energy marsh coasts with waves up to 1 m, waves are attenuated by more than 10% (and up to 50%) for E. athericus, which can be considered a conservative wave-attenuation estimator for salt marshes generally (Extended Data Fig. 1). Attenuation at high-energy marsh coasts (wave height > 1 m) does not exceed 10%. This wave attenuation functionality is also found in seagrass environments under low-energy conditions34, and may also apply in freshwater settings32. Decreasing salinity, towards brackish and fresh water marshes, induces an increase in species diversity, because species diversity increases with decreasing environmental stress33. It also leads to a shift towards species with longer and less flexible stems compared to E. athericus, such as the common reed Phragmitis australis35,36. Both higher species diversity and the shift to longer and less flexible stems enhance wave attenuation, even under higher vegetation damage. This agrees with the result of our sensitivity analysis (Extended Data Figs. 3–6).
Across multi-year to decadal timescales, salt marshes could drown due to sea level rise and/or limited sediment supply37 and lateral marsh retreat may take place due to cliff erosion38. As a result, ecosystem services, such as carbon storage and wave attenuation, could be diminished. Between the years 2000 and 2019, a substantial salt marsh area has been lost globally (719 km2), with main hotspots including the US Atlantic coast and the Gulf of Mexico39. Drivers of marsh loss are similar to drivers of vegetation damage and a decreasing wave attenuating capacity, that is, hydrodynamic exposure. For the aforementioned regions, our global analysis shows considerable vegetation damage due to long exposure duration (Fig. 4 and Extended Data Fig. 2). An increased vulnerability of coastal regions where marshes are retreating can thus be expected, as wave attenuation may also decline, further accelerating exposure of the coast.
Our results emphasize that restoration and conservation of salt marshes as a Nature-based Solution, supporting biodiversity, protect against extreme storms more effectively at low-energy coasts than at high-energy coasts. Hence, application at low-energy coasts should be prioritized, but even at high-energy coasts potential cost reduction is considerable as preventing 1 km dike heightening by 0.2 m, already saves 1.4 million USD2005 purchasing power parity, because of reduced overtopping rates29,40,41. Furthermore, reduction of the wave height by decimetres, offsets predicted average sea level rise of 0.49 m in 2100 (RCP4.5) already by decades42. This cost reduction can motivate continuous support and maintenance that is required for salt marshes to prevent long-term erosion and guarantee their persistence at high-energy coasts. The potential for wave attenuation emphasized by our results support a plea to protect marshes where they are currently present, and to restore former salt marshes, where fitting, to enhance their contribution to flood protection.
Methods
Large-scale assessment of vegetation breakage and wave attenuation
The Delta Flume and the physical model
The physical model was built in the Delta Flume (a wave flume located at Deltares) by transplanting salt marsh blocks on top of a sand bed with drainage pipes. An artificial dike with a slope of 1:3.6 was constructed at the back. The Delta Flume has a length of 300 m, a width of 5 m and a depth of 9.5 m. We used 66 salt marsh blocks to construct two 71-m-long and 2.0–2.2 m-wide salt marsh profiles. In between the two rows a path was constructed 5 cm below the surface of the marsh, to drain both marsh profiles and enable access, maintenance and (manual) measurements. The height difference between the path and marsh surface was comparable with the variations in the vegetated marsh, that is, the clay heights and the vegetation height.
Blocks with a depth of approximately 0.7 m were installed at the expected erosion-prone areas: six at the seaward salt marsh edge and two at the dike toe. In between these, 25 blocks with a depth of approximately 0.4 m were installed. To connect the dike slope to the marsh, a block with a depth of 0.4 m was also installed (Fig. 1). The seaward edge of the salt marsh had an elevation difference of 0.6 m with the artificial bare tidal flat to recreate field conditions with a cliff. A brushwood dam was used as edge protection at this seaward edge of the salt marsh—similar to field locations in the Wadden Sea area43,44,45 and other regions46—to prevent lateral erosion, enabling comparison with experimental runs. The bare tidal flat was constructed using concrete to prevent bed level dynamics at the flat, which could potentially affect the incoming wave at the marsh edge. The first 40 m of the bare tidal flat had a decreasing gradient of 1:45, followed by a gradient of 1:9 over 12.5 m to create a smooth transition to the flume bottom and to save material.
Transplanting salt marsh blocks
The salt marsh blocks were collected in the field at nature reserve Peazemerlannen at the mainland Wadden Sea coast (53° 24′ 19.0908″ N, 6° 5′ 58.3476″ E) in the Netherlands. The blocks were harvested at the end of the growing season in September and October 2023. Two locations, landward and seaward, were selected with different soil compositions. The median grain size, D50, was 0.013 ± 0.010 mm (0.003 ± 0.001 mm) and the clay content was 31.4 ± 6.8% (44.5 ± 4.8%) for the seaward (landward) location (Extended Data Table 1). The particle size distribution was determined by adding a peptisator to prevent flocculation to the dried sample. The solution is left to soak for 16 h and subsequently sieved over a 63 μm sieve. The fraction larger than 63 μm was mechanically sieved over a set of sieves ranging from 63 μm to 63 mm. The particles left on each sieve were weighed and processed to determine the distribution. The smaller fraction was analysed using a sedigraph. The smaller and larger fraction together determine the full distribution.
The above-ground vegetation was similar at both selected locations to prevent vegetation gradients in the physical model. The high marsh zone was selected, as the high marsh generally contributes most to wave attenuation due to the high bed elevation15. Elymus athericus was the vegetation species dominantly present, with a mix of Atriplex spp. and Aster tripolium.
The salt marsh blocks were harvested by pushing a mould of 2 × 2 m2 (0.7 m depth) or 2.2 × 2.2 m2 (0.4 m depth) into the ground. The area around the mould was dug out using a 35-to-50 tonne excavator. A steel-bottom plate was then slid under the mould to minimiuze disturbance of the vegetation and the marsh substrate within the mould by as much as possible. Subsequently, the 3,000 to 6,000 kg marsh blocks were lifted, deployed on a closed truck to prevent wind damage, and then transported to the Delta Flume.
The harvest location was elevated above spring tide to assure safe access over land. To work safely and minimize disturbances to the ecosystem, the harvest was executed after the breeding season and before the storm season, during daylight, in the shortest period possible. Temporary steel road plates were used to distribute the weight of the excavator and trucks, which minimized damage to the marsh.
After arrival near the Delta Flume, drainage holes were drilled into the boxes around the blocks. The blocks were continuously monitored visually and saturation (by measuring weight) and salinity were periodically measured in a sub-selection of the blocks. Blocks were irrigated during dry periods after the weight dropped. From December 2023 onwards, the blocks were installed in the physical model of the Delta Flume. After installation, artificial light from growing lights was applied to the part of the physical model covered by a hall, to balance the blocked supply of sunlight. Ventilation was also applied to create a more natural air flow.
Organic matter content and root biomass of the substrate
Mean organic matter content in the salt marsh substrate in our experiment was 4.7% ± 1.7% and ranged between 2.3% and 7.6% (Extended Data Table 1). Organic matter content was determined using loss-on-ignition. The organic matter content in the substrate in our experiment is similar to many other European salt marshes, which typically range between 0 and 76.7% (mean of 8.5%)47. More specifically, studies in the Wadden Sea, Northwestern Europe show a range between 1.3% and 8.8% (mean of 4.2%)48 and in the Mediterranean between 4% and 30% (ref. 49). The organic matter content in our study is within the lower range when comparing to, for example, North American marshes, which are more organic-rich (range 0−55%)50.
Prior studies describe a rooting depth of vegetation species in salt marshes of 10 to 40 cm below the surface51. The E. athericus marsh cover has a web-like root structure (that is, dichotomous branching), with long roots compared to other species, but an average to low central root and branch density52. Vegetation roots stabilize the soil, potentially with increasing stability if the vegetation composition is more diverse53. Root mass in our experiment was measured at 5, 10 and 20 cm depth, with n (sample size) = 4. Root samples were collected after the experimental wave runs at locations where the soil was undisturbed by placing bulk density rings (6 cm diameter and 4.05 cm depth), with the midpoint at the chosen depth. The rings with material were carefully dug out, roots were gently rinsed and dried in an oven at 60 °C for 48 h, before weighing to obtain the dry root mass (g) at each depth interval. The root density was then calculated. Below-ground biomass was mainly present in the top layer in our experiment (5 cm; 78% of the total biomass; Extended Data table 2).
Our study generally implies that ecosystem services that depend on the stability of the salt marsh substrate, including wave attenuation and carbon storage54,55, are unlikely to be affected by surface erosion during extreme storms, as the marsh substrate remains stable both at low- and high-energy coasts. This conclusion is based on our flume experiment, which contains two soil types (Extended Data table 1). The organic matter content of the soil is representative for European marshes, which corresponds to the lower range of the organic-rich soils on the US East Coast and the Gulf of Mexico (Methods)50. Our experiment provides evidence for the erosion resistance of soils; however, soil parameters, and in turn erosion resistance56, vary globally, emphasizing the need for controlled erosion experiments under extreme storms with a range of established and restored marsh soils. Organic-rich soils can have a more open structure that might result in instability51, and also brackish and freshwater marshes might be more prone to erosion due to shallower root zones and potentially low inorganic sediment content21. Hence, our projection yields a conservative estimate regarding soil erodibility for salt marshes, but may overestimate the stability of organic-rich soils and brackish marshes.
The experiment
The experimental runs in the wave flume started in February 2024 to conservatively test the vegetation in its winter state. The state of the marsh vegetation installed in the Delta Flume before starting the experimental runs was equal to vegetation in the field, both measured in February 2024 (Fig. 2).
The experimental programme included three different water levels (1.5 m, 2.5 m and 4.0 m at the marsh, which correspond to 4.4 m, 5.4 m and 6.9 m at the wave paddle, respectively). The water levels were coupled with three significant wave heights (0.75 m, 1.25 m and 2.00 m; JONSWAP wave spectrum), maximizing the ratio of wave height and water depth at the marsh platform57,58. Smaller wave heights, with similar water depths (hence decreasing the wave height to water depth ratio) will result in a decreasing contribution to wave attenuation, but also less vegetation damage5. It may be expected that under these conditions the wave height at the landward side will always be smaller than under the most conservative wave height to water depth ratio we tested, as there is a limit of wave attenuation by vegetation with an increasing wave height to water depth ratio5. So, we aimed at the most conservative wave height to water depth ratio cases, enhancing vegetation damage and potentially decreasing wave attenuation by vegetation. Furthermore, two different values for wave steepness (0.04 and 0.02) were tested. These settings were combined in an experimental program with increasing water depths and significant wave heights over time, potentially resulting in increasing damage. First a short test (approximately 100 waves) was performed with water depths of 1.5 m and 2.5 m, to test the stability of the marsh, and subsequently longer tests (approximately 1,000 waves) with increasing water depths and wave heights were applied (Supplementary Table 1). This sequence was executed three times to study marsh stability and wave attenuation under potentially increasing vegetation damage: (1) light vegetation damage; (2) substantial vegetation damage; and (3) removed above-ground vegetation (Supplementary Table 1). This allowed us to explicitly quantify wave attenuation by vegetation as a result of progressive damage of the above-ground biomass, by subtracting wave attenuation by the marsh elevation in experimental runs without above-ground biomass (percentage decrease of Hm0) from wave attenuation in runs with full and damaged vegetation. Before the last repetition all vegetation was mowed level with the surface, to test wave attenuation under extreme vegetation damage potential. A significant wave height was also applied, approximating the maximum significant wave height tested by Möller et al.5, to facilitate comparison with that study (refer to Supplementary Table 1 for the full experimental program). The full range of tested wave heights allows us to generalize our findings.
Waves were forced with a wave paddle equipped with an active reflection compensation. The water level elevation in front of the wave paddle was continuously measured to observe the wave field including reflected waves. The motion of the wave paddle compensates for reflected waves to avoid reflection back into the physical model. The reflection coefficient in deep water varies between 0.2 (low waves and 4% wave steepness; experimental run SM-01 in Supplementary Table 1) and 0.35 (high waves and 2% wave steepness; experimental run SM-14 in Supplementary Table 1).
Wave flume measurements and data processing
The clay surface was measured at 32 fixed locations at the salt marsh (16 per transect) using a total station (Trimble Ri) that has a measurement accuracy of 2 mm. The concrete bare tidal flat, seaward from the salt marsh in the flume, was not subject to change. Measurements were taken daily or bi-daily and bed-level-changes (mean, s.d. and standard error) were calculated for each measurement (Extended Data Fig. 7). The s.d. (43 to 48 mm) of all 32 measurement locations exceeded the average bed level decrease over the full experiment (7 mm), highlighting that the surface decrease after 21 h of extreme wave forcing was smaller than typical elevations in the existing microtopography of the marsh (Extended Data Fig. 7).
Vegetation properties were quantified using destructive measurements (bi)daily after changing the significant wave height and daily non-destructive measurements, by (1) measuring the highest and lowest vegetation canopy height at six locations, corresponding to separate salt marsh blocks (n = 6). The canopy height was measured by carefully lowering a styrofoam plate (30 cm diameter) with a hole over a stick. Height measurements were taken after the plate was lying stably at the canopy; (2) measurements of vegetation biomass (n = 6) by collecting all above-ground biomass from a square surface of 20 × 20 cm2, taking wet weight, drying in the oven for two weeks at 65 °C and taking dry weight; (3) measuring stem characteristics (E. athericus) by randomly selecting 20 standing stems from the marsh (n = 20). The length of each stem and outer diameter 5 cm above the base were measured using a caliper; (4) measuring total biomass removal (that is, flotsam) due to wave exposure by collecting all vegetation material at the dike and in the water with a fishing net made from chicken wire. Total wet weight was measured, and subsequently a wet subsample was taken and weighed. The wet subsample was dried for two weeks at 65 °C in an oven, whereafter the dry weight was taken; (5) measuring stem characteristics from already broken stems in the flotsam by randomly collecting 20 stems (E. athericus) from the flotsam after experimental runs. Subsequently, length and diameter were measured analogously to the standing stems, and flexural strength was measured. The destructive measurements for biomass (vegetation measurement 2) and stem length (vegetation measurement 3) affected a marsh area less than 1% of the total salt marsh in the physical model.
Vegetation stems (E. athericus) were collected in the field at the seaward and landward location (n = 75) where the salt marsh blocks were harvested. Stems were collected in February 2024 at the start of the experiment to allow comparison of the development of vegetation next to and in the flume with that in the field.
Vegetation stem length and dry biomass measurements were post-processed by calculating the mean, median, quartiles, inter-quartile range and standard error (Figs. 2 and 3). An exponential decay function was then fitted (Fig. 3), and then used to quantify vegetation damage over exposure time. Wave attenuation was related to stem length per wave height class, that is, significant wave heights of 0.75 m (r2 = 0.89), 1.25 m (r2 = 0.57) and 2.00 (r2 = 0.33; Fig. 3). Significant differences between above-ground biomass in the field and flume at the start of the experiment were tested using a Mann–Whitney U test. Significant differences in increasingly damaged vegetation height and biomass were tested using a t-test for normal and Mann–Whitney U test for non-normally distributed samples with a Benjamini–Hochberg FDR P-value correction. Significant differences over the total experiment were tested using a Welch t-test with Benjamini–Hochberg false-discovery rate (FDR) P-value correction. The few statistical differences might have been caused by the high variability of stem height and above-ground biomass at the marsh, and for the latter also the limited number of replicates to damage the marsh as little as possible.
Wave characteristics were measured using fixed resistance-type wave gauges present in the Delta Flume at the left wall of the flume (looking from the wave paddle to the end of the flume) with a measurement accuracy smaller than 1 cm (ref. 59). No variations in the width direction were discernible during experimental runs, because the setup was symmetrical in the width direction. We assume no variations in width, as is the case in general for flumes (as width, 5 m « length, 300 m)60. For every experiment, Hm0 is determined in front of and at the landward end of the marsh by using the three wave gauges in front of the marsh (locations X = 40.5, 43.5 and 49.5 m; Fig. 1) and at the end of the marsh (locations X = 151.4, 159.1 and 160.8 m; Fig. 1). Zelt and Skjelbreia's method, using three wave height meters, was used to separate incoming and reflected waves61. Hereafter, the difference in wave height in front of the marsh and at the landward end of the marsh was calculated. Subsequently, wave attenuation was quantified. The explicit contribution of vegetation was quantified by calculating the difference in wave attenuation for the experiments with (Supplementary Table 1; experiment SM-1–29) and without (Supplementary Table 1; experiment SM-30–37) vegetation. Wave attenuation by vegetation was calculated as the relative share of the incoming wave to enable comparison of different experimental runs and global scenarios.
Calculating the global contribution of breaking vegetation
Development of the statistical model
The global contribution of breaking vegetation to wave attenuation is explored by a parameterization where wave attenuation is a response variable of the predictor variables exposure duration and incoming wave height. The assessed E. athericus (also Elytrigia atherica) is widespread in Northwestern European salt marshes, appearing in for example, Denmark, Germany, the Netherlands, United Kingdom, France and Portugal (Extended Data Fig. 1). Stem height decrease of E. athericus through exposure duration in this large scale experiment (Fig. 3) is used as a conservative estimator of wave attenuation by above-ground vegetation under the most severe conditions (water depth to wave height ratio of 0.5).
To explore the contribution of salt marsh vegetation to wave attenuation globally, a GLM is applied with a Tweedie distribution and a log link function enabling the use of zeros and positive continuous data and proportional effects (for example, exponential decrease of wave attenuation with increasing exposure duration). The GLM is a strong predictor of the variability of wave attenuation by vegetation (pseudo-R2 = 0.97). Wave attenuation by vegetation decreased with increasing incoming wave height (β = −1.3258, SE = 0.185, z = −7.16, P < 0.001) and longer exposure duration (β = −0.0494, SE = 0.011, z = −4.42, P < 0.001). The GLM including incoming wave height and exposure duration is a globally significant predictor compared with the null intercept-only model (χ² = 59.26, df = 2, P < 0.001).
Stem height in salt marshes as proxy for wave attenuation
Key for the functionality of the marsh is the presence of salt-tolerant vegetation (halophytes), such as herbs, grasses and shrubs, which typically depend on salinity and inundation gradients4. The stem height of the vegetation is an important parameter for wave attenuation. Stem height is used as a proxy for wave attenuation as penetration of the stem in the water column is considered a strong predictor of wave attenuation, especially under extreme wave heights and water levels13. As a result, damage to vegetation by a decreasing stem height will have a direct impact on wave attenuation. The stem height and biomass of E. athericus are comparable with global marsh vegetation species that carry stems. At the end of our experiment, both the values of the damaged stem height and biomass were lower than global values for (other) salt marsh vegetation species (Extended Data Fig. 1) throughout the year.
Increasing wave attenuation with stem height can be expected both at low- and high-energy coasts, and is also found as a result of the flume experiment (Fig. 3). Yet for high-energy conditions, the higher risk of damage may cancel this benefit. Comparing Elymus with Spartina spp., locally a species growing at a lower elevation and regionally a dominant species in, for example, North America62,63, wave-induced damage to Spartina spp. is lower due to a higher flexibility26. Hence, attenuation can be expected to be higher as more stems and biomass persists (Fig. 3). Attenuation can also be expected to increase towards a lower salinity environment, since due to decreasing environmental stress, species diversity increases32,33,64.
70% of the salt marshes globally present are found in the temperate climate zone and therefore experience a winter season31. In general, the vegetation state at the end of the winter can be considered to yield a conservative estimate for vegetation stem height, as vegetation outside the winter season, for example, in the growing season, is more resistant26. Nevertheless, vegetation will be damaged during extreme storms, also when being more resistant early in the winter season, and might reduce wave attenuation during consecutive storms. Furthermore, E. athericus in our experiment can be considered to yield a conservative estimate of wave attenuation, because its breaking force is relatively weak compared to other salt marsh vegetation species35. Less vegetation damage leads to longer stems persisting and hence a higher wave attenuation capacity. In addition to this, we tested a single salt marsh zone, whereas salt marshes in general contain multiple zones that enhance the wave attenuation capacity65. Finally, only a small (70 m) part of the marsh was considered for wave attenuation. Our experiment enables future site-specific assessments of wave attenuation through vegetation height. These quantifications require extensive vegetation characterization (for example, spatiotemporal variable height). Effective methods for mapping vegetation heights are available through remote sensing, for example: high-resolution satellite imagery, LiDAR and Photogrammetry66,67,68. However, these techniques still require extensive field validation, especially if vegetation composition is variable.
Global datasets to determine salt marsh transects and wave exposure
Global wave attenuation along salt marsh foreshores is estimated by using global data layers as input for the statistical model. The approach to derive coastal profile data is based on a previous global study focused on wave-attenuation on vegetated foreshores29. We incorporated several updates: (1) elevation data from DeltaDTM was used30 instead of MERIT69 and vegetation extent data was updated31; (2) we filtered foreshores that are preceded by waterbodies with a minimal length of 1 km using a global water mask70 to assure that foreshore data are derived at the right location; (3) salt marsh areas sheltered behind higher landscape features, such as dunes, were excluded by flagging vegetation presence as false if the mean elevation in the vegetated zone is lower than the mean elevation of the preceding non-vegetated foreshore data points; and (4) false positives of vegetation presence in areas with steep transitions (for example, steep coastal slopes or cliffs) were corrected by applying an Interquartile Range filter on elevation within vegetated areas with a multiplier of 1.5. In general, this filtering resulted in an equal reduction across continents.
Following our experiment, nearshore waves at the seaward salt marsh edge are estimated to be 50% of the water depth, slightly lower than 55% estimated for very flat nearshore areas29,57,58. Using the global datasets, exposure duration during a single storm with a recurrence time (RPS) of 100 to 1,000 years was calculated for 1 km spaced transects where salt marsh vegetation is present.
Next, we combined the derived elevation profiles, salt marsh extents and significant wave heights with global storm tide hydrographs28, based on Euclidean distance, to calculate inundation depths and consequential exposure duration. Globally observed peak water levels (exceeding 1 m water depth) at the globally derived salt marsh locations remain for the larger part (around 90%) within the water level range applied in the wave flume. Globally observed exposure duration with water levels exceeding the threshold of 1.0 m (with Hm0 of 0.5 m) did not exceed 1,000 min (16.67 h), which is within the duration of the flume experiment (21 h). Subsequently, this information is used to calculate vegetation damage, specifically the expected decrease in stem height. As stem height damage in the Delta Flume experiment started already during the most tranquil hydrodynamic conditions (h = 1.50 m; Hm0 = 0.75 m), the initiation of stem height damage in the global model was set following previous controlled flume experiments28. In those previous experiments, which started at water depths of 1 m and wave heights of 0.1 m, the first significant stem damage was observed after water depths of 1 m and wave heights of 0.5 m on average27. Using the local storm surge hydrographs, exposure duration for vegetation damage is calculated over the time window during which wave heights at the marsh exceed 0.5 m from the start of the storm until the point in time when the highest waves occur, that is, at the peak of the storm surge hydrograph. The maximum incoming wave height at the marsh edge is calculated at the peak of the storm, with the most severe estimate for the wave height being 50% of the water depth29,57,58. Finally, wave attenuation at the peak of the storm is calculated using the GLM, as potentially the highest depth-limited waves occur at this point.
Data availability
Experimental data from this study are available via https://doi.org/10.4121/112edd27-1dd3-4ba3-b5cd-8d15d7fed39f. Global storm surge hydrographs from ref. 28, used in this study, are available at https://doi.org/10.4121/21270948. The tidal elevation profiles updated by ref. 29 are available at https://doi.org/10.5281/zenodo.2525658.
Code availability
All general-purpose software packages that we used are open source: Python v.3.12 (https://www.python.org/), NumPy v.1.26.4 (https://numpy.org/), Pandas v.2.2.2 (https://pandas.pydata.org/docs/index.html#), GeoPandas v.1.0.1 (https://geopandas.org/en/stable/), NetCDF4 v.1.6.2 (https://pypi.org/project/netCDF4/), Xarray v.2023.6.0 (https://docs.xarray.dev/en/stable/). For statistical testing, SciPy v.1.13.1 (https://scipy.org/); scikit-learn or sklearn v.1.4.2 (https://scikit-learn.org/stable/); and statsmodels v.0.14.2 (https://www.statsmodels.org/stable/index.html) were used. For plotting and creating maps Matplotlib v.3.8.4 (https://matplotlib.org/), Seaborn v.0.13.2 (https://seaborn.pydata.org/), contextily v.1.6.2 (https://contextily.readthedocs.io/en/latest/), Cartopy v.0.24.0 (https://pypi.org/project/Cartopy/) and shapely v.2.0.5 (https://pypi.org/project/shapely/) were used. The code written specifically for this project to analyse vegetation data and apply the global analysis is available at https://doi.org/10.4121/112edd27-1dd3-4ba3-b5cd-8d15d7fed39f.
References
Temmerman, S. et al. Ecosystem-based coastal defence in the face of global change. Nature 504, 79–83 https://doi.org/10.1038/nature12859 (2013).
van Wesenbeeck, B. K. et al. Damming deltas: a practice of the past? Towards nature-based flood defenses. Estuar. Coast. Shelf Sci. 140, 1–6 https://doi.org/10.1016/j.ecss.2013.12.031 (2014).
Borsje, B. W. et al. How ecological engineering can serve in coastal protection. Ecol. Eng. 37, 113–122 https://doi.org/10.1016/j.ecoleng.2010.11.027 (2011).
Adam, P. Saltmarsh Ecology (Cambridge Univ. Press, 1993).
Möller, I. et al. Wave attenuation over coastal salt marshes under storm surge conditions. Nat. Geosci. 7, 727–731 https://doi.org/10.1038/ngeo2251 (2014).
Marin-Diaz, B. et al. Using salt marshes for coastal protection: effective but hard to get where needed most. J. Appl. Ecol. 60, 1286–1301 https://doi.org/10.1111/1365-2664.14413 (2023).
Vuik, V., Borsje, B. W., Willemsen, P. W. J. M. & Jonkman, S. N. Salt marshes for flood risk reduction: quantifying long-term effectiveness and life-cycle costs. Ocean Coast. Manag. 171, 96–110 https://doi.org/10.1016/j.ocecoaman.2019.01.010 (2019).
Caldera, G., Stolle, J., Pham Van Bang, D., Murphy, E. & Knox, P. Seasonal and inter-annual changes in wave attenuation by a constructed salt marsh on a sloping bed. Ecol. Eng. 221, 107758 https://doi.org/10.1016/j.ecoleng.2025.107758 (2025).
Leonardi, N. et al. Dynamic interactions between coastal storms and salt marshes: a review. Geomorphology 301, 92–107 https://doi.org/10.1016/j.geomorph.2017.11.001 (2018).
Wamsley, T. V., Cialone, M. A., Smith, J. M., Atkinson, J. H. & Rosati, J. D. The potential of wetlands in reducing storm surge. Ocean Eng. 37, 59–68 https://doi.org/10.1016/j.oceaneng.2009.07.018 (2010).
Hu, K., Chen, Q. & Wang, H. A numerical study of vegetation impact on reducing storm surge by wetlands in a semi-enclosed estuary. Coast. Eng. 95, 66–76 https://doi.org/10.1016/j.coastaleng.2014.09.008 (2015).
Zhu, Z. et al. Historic storms and the hidden value of coastal wetlands for nature-based flood defence. Nat. Sustain. 3, 853–862 https://doi.org/10.1038/s41893-020-0556-z (2020).
Vuik, V., Suh Heo, H. Y., Zhu, Z., Borsje, B. W. & Jonkman, S. N. Stem breakage of salt marsh vegetation under wave forcing: a field and model study. Estuar. Coas. Shelf Sci. 200, 41–58 https://doi.org/10.1016/j.ecss.2017.09.028 (2018).
Willemsen, P. W. J. M., Borsje, B. W., Vuik, V., Bouma, T. J. & Hulscher, S. J. M. H. Field-based decadal wave attenuating capacity of combined tidal flats and salt marshes. Coast. Eng. 156, 103628 https://doi.org/10.1016/j.coastaleng.2019.103628 (2020).
Vuik, V., Jonkman, S. N., Borsje, B. W. & Suzuki, T. Nature-based flood protection: the efficiency of vegetated foreshores for reducing wave loads on coastal dikes. Coastal Eng. 116, 42–56 https://doi.org/10.1016/j.coastaleng.2016.06.001 (2016).
Pannozzo, N., Leonardi, N., Carnacina, I. & Smedley, R. Salt marsh resilience to sea-level rise and increased storm intensity. Geomorphology 389, 107825 https://doi.org/10.1016/j.geomorph.2021.107825 (2021).
Dullaart, J. C. M. et al. Accounting for tropical cyclones more than doubles the global population exposed to low-probability coastal flooding. Commun. Earth Environ. 2, 135 https://doi.org/10.1038/s43247-021-00204-9 (2021).
Muis, S. et al. Global projections of storm surges using high-resolution CMIP6 climate models. Earth’s Future 11, e2023EF003479 https://doi.org/10.1029/2023EF003479 (2023).
Garzon, J. L., Maza, M., Ferreira, C. M., Lara, J. L. & Losada, I. J. Wave attenuation by spartina saltmarshes in the chesapeake bay under storm surge conditions. J. Geophys. Res. Oceans 124, 5220–5243 https://doi.org/10.1029/2018JC014865 (2019).
Spencer, T. et al. Salt marsh surface survives true-to-scale simulated storm surges. Earth Surf. Processes Landforms 41, 543–552 https://doi.org/10.1002/esp.3867 (2016).
Howes, N. C. et al. Hurricane-induced failure of low salinity wetlands. Proc. Natl Acad. Sci. USA 107, 14014–14019 https://doi.org/10.1073/pnas.0914582107 (2010).
Gijsman, R. et al. Nature-based engineering: a review on reducing coastal flood risk with mangroves. Front. Mar. Sci. 8, 2021 https://doi.org/10.3389/fmars.2021.702412 (2021).
Morton, R. A. & Barras, J. A. Hurricane impacts on coastal wetlands: a half-century record of storm-generated features from Southern Louisiana. J. Coast. Res. 27, 27–43 https://doi.org/10.2112/JCOASTRES-D-10-00185.1 (2011).
Bouma, T. J. et al. Identifying knowledge gaps hampering application of intertidal habitats in coastal protection: opportunities & steps to take. Coastal Eng. 87, 147–157 https://doi.org/10.1016/j.coastaleng.2013.11.014 (2014).
Mason, V. G. et al. Identifying small-scale gradients in sediment stability as early indicators of saltmarsh cliff Initiation. J. Geophys. Res. Earth Surface 130, e2025JF008297 https://doi.org/10.1029/2025JF008297 (2025).
Reents, S. et al. Species-specific and seasonal differences in the resistance of salt-marsh vegetation to wave impact. Front. Mar. Sci. 9, 2022 https://doi.org/10.3389/fmars.2022.898080 (2022).
Rupprecht, F. et al. Vegetation-wave interactions in salt marshes under storm surge conditions. Ecol. Eng. 100, 301–315 https://doi.org/10.1016/j.ecoleng.2016.12.030 (2017).
Dullaart, J. C. M. et al. Enabling dynamic modelling of coastal flooding by defining storm tide hydrographs. Nat. Hazards Earth Syst. Sci. 23, 1847–1862 https://doi.org/10.5194/nhess-23-1847-2023 (2023).
van Zelst, V. T. M. et al. Cutting the costs of coastal protection by integrating vegetation in flood defences. Nat. Commun. 12, 6533 https://doi.org/10.1038/s41467-021-26887-4 (2021).
Pronk, M. et al. DeltaDTM: a global coastal digital terrain model. Sci. Data 11, 273 https://doi.org/10.1038/s41597-024-03091-9 (2024).
Worthington, T. A. et al. The distribution of global tidal marshes from Earth observation data. Global Ecol. Biogeogr. 33, e13852 https://doi.org/10.1111/geb.13852 (2024).
Ren, J. et al. Wave-attenuation characteristics of combined-vegetation wave break forests for big rivers with large flood water level changes. Water Sci. Technol. 83, 831–840 https://doi.org/10.2166/wst.2021.011 (2021).
Więski, K., Guo, H., Craft, C. B. & Pennings, S. C. Ecosystem functions of tidal fresh, brackish, and salt marshes on the Georgia coast. Estuaries Coasts 33, 161–169 https://doi.org/10.1007/s12237-009-9230-4 (2010).
Bradley, K. & Houser, C. Relative velocity of seagrass blades: implications for wave attenuation in low-energy environments. J. Geophys. Res. Earth Surface 114, https://doi.org/10.1029/2007JF000951 (2009).
Zhu, Z., Yang, Z. & Bouma, T. J. Biomechanical properties of marsh vegetation in space and time: effects of salinity, inundation and seasonality. Ann. Botany 125, 277–290 https://doi.org/10.1093/aob/mcz063 (2019).
Dijkema, K. S. Salt and brackish marshes around the Baltic Sea and adjacent parts of the North Sea: their vegetation and management. Biol. Conserv. 51, 191–209 https://doi.org/10.1016/0006-3207(90)90151-E (1990).
Fagherazzi, S. et al. Salt marsh dynamics in a period of accelerated sea level rise. J. Geophy. Res. Earth Surface 125, e2019JF005200 https://doi.org/10.1029/2019JF005200 (2020).
Leonardi, N., Ganju, N. K. & Fagherazzi, S. A linear relationship between wave power and erosion determines salt-marsh resilience to violent storms and hurricanes. Proc. Natl Acad. Sci. USA 113, 64–68 https://doi.org/10.1073/pnas.1510095112 (2016).
Campbell, A. D., Fatoyinbo, L., Goldberg, L. & Lagomasino, D. Global hotspots of salt marsh change and carbon emissions. Nature 612, 701–706 https://doi.org/10.1038/s41586-022-05355-z (2022).
Ward, P. J. et al. A global framework for future costs and benefits of river-flood protection in urban areas. Nat. Clim. Change 7, 642–646 https://doi.org/10.1038/nclimate3350 (2017).
Pullen, T. et al. EurOtop wave overtopping of sea defences and related structures: assessment manual. 2007.
DeConto, R. M. & Pollard, D. Contribution of Antarctica to past and future sea-level rise. Nature 531, 591–597 https://doi.org/10.1038/nature17145 (2016).
Hofstede, J. L. Integrated management of artificially created salt marshes in the Wadden Sea of Schleswig-Holstein, Germany. Wetlands Ecol. Manage. 11, 183–194 https://doi.org/10.1023/A:1024248127037 (2003).
Bakker, J., P. Esselink, R. Van der Wal & Dijkema, K. Options for restoration and management of coastal salt marshes in Europe. Restoration Ecol. Sustain. Develop. 286–322 https://hdl.handle.net/11370/ebfebc55-c354-45d9-b294-3fe9f0043359 (1997).
Willemsen, P. W. J. M., et al. Facilitating salt marsh restoration: the importance of event-based bed level dynamics and seasonal trends in bed level change. Front. Marine Sci. https://doi.org/10.3389/fmars.2021.793235 (2022).
Provan, M., E. Murphy, A. Rahman, E. Morris & Matfin, A. Large-scale experimental model of edge treatments for constructed salt marshes. In Proc. 9th Conference on Physical Modelling in Coastal Engineering https://doi.org/10.59490/coastlab.2024.748 (2024).
Graversen, A. E. L. et al. A marine and salt marsh sediment organic carbon database for European regional seas (EURO-CARBON). Data Brief 60, 111595 https://doi.org/10.1016/j.dib.2025.111595 (2025).
Mittmann-Goetsch, J., Wilson, M., Jensen, K. & Mueller, P. Root-driven soil reduction in wadden sea salt marshes. Wetlands 44, 112 https://doi.org/10.1007/s13157-024-01867-8 (2024).
Puppin, A. et al. Spatial patterns of organic matter content in the surface soil of the salt marshes of the Venice Lagoon (Italy). Biogeosciences 21, 2937–2954 https://doi.org/10.5194/bg-21-2937-2024 (2024).
Turner, R. E., Swenson, E. M. & Milan, C. S. in Concepts and Controversies in Tidal Marsh Ecology (eds Weinstein, M. P. & Kreeger, D. A.) 583–595 (Springer, 2000).
Brooks, H. et al. Resistance of salt marsh substrates to near-instantaneous hydrodynamic forcing. Earth Surf. Processes Landforms 46, 67–88 https://doi.org/10.1002/esp.4912 (2021).
Bouma, T. J., Nielsen, K. L., Van Hal, J. & Koutstaal, B. Root system topology and diameter distribution of species from habitats differing in inundation frequency. Funct. Ecol. 15, 360–369 https://doi.org/10.1046/j.1365-2435.2001.00523.x (2001).
Ford, H., Garbutt, A., Ladd, C., Malarkey, J. & Skov, M. W. Soil stabilization linked to plant diversity and environmental context in coastal wetlands. J. Veget. Sci. 27, 259–268 https://doi.org/10.1111/jvs.12367 (2016).
Mason, V. G. et al. Blue carbon benefits from global saltmarsh restoration. Global Change Biol. 29, 6517–6545 https://doi.org/10.1111/gcb.16943 (2023).
Mcleod, E. et al. A blueprint for blue carbon: toward an improved understanding of the role of vegetated coastal habitats in sequestering CO2. Front. Ecol. Environ. 9, 552–560 https://doi.org/10.1890/110004 (2011).
Feagin, R. A. et al. Does vegetation prevent wave erosion of salt marsh edges?. Proc. Natl Acad. Sci. USA 106, 10109–10113 https://doi.org/10.1073/pnas.0901297106 (2009).
Massel, S. R. On the largest wave height in water of constant depth. Ocean Eng. 23, 553–573 https://doi.org/10.1016/0029-8018(95)00049-6 (1996).
Nelson, R. C. Depth limited design wave heights in very flat regions. Coastal Eng. 23, 43–59 https://doi.org/10.1016/0378-3839(94)90014-0 (1994).
Wenneker, I., Hoffmann, R. & Hofland, B. Wave generation and wave measurements in the new delta flume. In 6th International Conference on the Application of Physical Modelling in Coastal and Port Engineering and Science https://resolver.tudelft.nl/uuid:2f7bd338-afb8-432f-856a-d2a3dd47fdc2 (2016).
Van Gent, M. R. A. Wave runup on dikes with shallow foreshores. J. Waterw. Port Coastal Ocean Eng. 127, 254–262 https://doi.org/10.1061/(ASCE)0733-950X(2001)127:5(254) (2001).
Zelt, J. A. & Skjelbreia, J. E. Estimating incident and reflected wave fields using an arbitrary number of wave gauges. In 23rd International Conference on Coastal Engineering https://doi.org/10.1061/9780872629332.058 (1992).
Pennings, S. C. & Bertness, M. D. Salt marsh communities. Mar. Commun. Ecol. 11, 289–316 (2001).
Bertness, M. D. Zonation of Spartina patens and Spartina alterniflora in New England salt marsh. Ecology 72, 138–148 https://doi.org/10.2307/1938909 (1991).
Schulte Ostermann, T. et al. Identifying key plant traits and ecosystem properties affecting wave attenuation and the soil organic carbon content in tidal marshes. Estuar. Coasts 47, 144–161 https://doi.org/10.1007/s12237-023-01266-y (2024).
Schoutens, K. et al. Biodiversity and self-organization improve wave attenuation by tidal marshes (manuscript in preparation).
Collin, A., Lambert, N. & Etienne, S. Satellite-based salt marsh elevation, vegetation height, and species composition mapping using the superspectral WorldView-3 imagery. Int. J. Remote Sens. 39, 5619–5637 https://doi.org/10.1080/01431161.2018.1466084 (2018).
Lee, E. I. H., Amin, S. & Nepf, H. Morphology-based correction improves plant height estimation from drone RGB SfM photogrammetry in dense salt marsh canopy. Remote Sens. Appl. Soc. Environ. 40, 101796 https://doi.org/10.1016/j.rsase.2025.101796 (2025).
Pinton, D., Canestrelli, A., Wilkinson, B., Ifju, P. & Ortega, A. Estimating ground elevation and vegetation characteristics in coastal salt marshes using UAV-based lidar and digital aerial photogrammetry. Remote Sens. 13, 4506 https://doi.org/10.3390/rs13224506 (2021).
Yamazaki, D. et al. A high-accuracy map of global terrain elevations. Geophys. Res. Lett. 44, 5844–5853 https://doi.org/10.1002/2017GL072874 (2017).
Pekel, J. F., Cottam, A., Gorelick, N. & Belward, A. S. High-resolution mapping of global surface water and its long-term changes. Nature 540, 418–422 https://doi.org/10.1038/nature20584 (2016).
Schulze, D., Rupprecht, F., Nolte, S. & Jensen, K. Seasonal and spatial within-marsh differences of biophysical plant properties: implications for wave attenuation capacity of salt marshes. Aquat. Sci. 81, 65 https://doi.org/10.1007/s00027-019-0660-1 (2019).
Darby, F. A. & Turner, R. E. Below- and above-ground Spartina alterniflora production in a Louisiana salt marsh. Estuaries Coasts 31, 223–231 https://doi.org/10.1007/s12237-007-9014-7 (2008).
Gao, J. H. et al. The effect of biomass variations of Spartina alterniflora on the organic carbon content and composition of a salt marsh in northern Jiangsu Province, China. Ecol. Eng. 95, 160–170 https://doi.org/10.1016/j.ecoleng.2016.06.088 (2016).
Tripathee, R. & Schäfer, K. V. R. Above- and below-ground biomass allocation in four dominant salt marsh species of the Eastern United States. Wetlands 35, 21–30 https://doi.org/10.1007/s13157-014-0589-z (2015).
Li, H., Shao, J., Qiu, S. & Li, B. Native Phragmites dieback reduced its dominance in the salt marshes invaded by exotic Spartina in the Yangtze River estuary, China. Ecol. Eng. 57, 236–241 https://doi.org/10.1016/j.ecoleng.2013.04.033 (2013).
Bart, D. & Hartman, J. M. Environmental determinants of Phragmites australis expansion in a New Jersey salt marsh: an experimental approach. Oikos 89, 59–69 https://doi.org/10.1034/j.1600-0706.2000.890107.x (2000).
Paquier, A.-E., Haddad, J., Lawler, S. & Ferreira, C. M. Quantification of the attenuation of storm surge components by a coastal wetland of the US mid atlantic. Estuar. Coasts 40, 930–946 https://doi.org/10.1007/s12237-016-0190-1 (2017).
Jadhav, R. S. & Chen, Q. Probability distribution of wave heights attenuated by salt marsh vegetation during tropical cyclone. Coast. Eng. 82, 47–55 https://doi.org/10.1016/j.coastaleng.2013.08.006 (2013).
Yang, S. L., Shi, B. W., Bouma, T. J., Ysebaert, T. & Luo, X. X. Wave attenuation at a salt marsh margin: a case study of an exposed coast on the Yangtze estuary. Estuar. Coasts 35, 169–182 https://doi.org/10.1007/s12237-011-9424-4 (2012).
Ysebaert, T. et al. Wave attenuation by two contrasting ecosystem engineering salt marsh macrophytes in the intertidal pioneer zone. Wetlands 31, 1043–1054 https://doi.org/10.1007/s13157-011-0240-1 (2011).
Acknowledgements
We would like to thank Rijkswaterstaat Noord-Nederland and It Fryske Gea for their permission and contribution to harvesting the salt marsh blocks. We would like to thank the Delta flume team, including S. Riedstra and G. Mourik from Deltares, E. Ozturk from the University of Twente, and P. van der Gaag, J. R. Monteiro, A. van der Vlies, A. Doorn and C. Willems from Delft University of Technology. Finally, we would like to thank Van Aalsburg and Aannemersbedrijf Jac. de Olde.
Funding
This research was supported by the ‘LIVING DIKES – Realising Resilient and Climate-Proof Coastal Protection’ project (with project number NWA.1292.19.257) of the NWA research program ‘Research on Routes by Consortia (ORC)’, which is funded by the Netherlands Organization for Scientific Research (NWO). The Delta Flume experiment was commissioned by Wetterskip Fryslân and funded by the Dutch Flood Protection Program (HWBP). Pim Willemsen and this research was further supported by the Dutch Research Council in the research project: “Salt marshes: where climate change adaptation meets climate change mitigation” (NWO-AES-VENI 2023; 21063). Bas Borsje, Sarah Dzimballa and Thomas van Veelen were supported by the research project: “LIVING ON THE EDGE: Using soft solutions to buffer coasts against extreme hydro-meteorological events” (NWO-AES-VIDI 2021; 18924), funded by the Dutch Research Council. Vincent van Zelst received funding from TKI Delta Technology (Topconsortia for Knowledge and Innovation) under the project entitled VINCARR, project number TU08.
Author information
Authors and Affiliations
Wageningen University & Research, Wageningen, the Netherlands
Pim W. J. M. Willemsen & Antonius J. F. Hoitink
Deltares, Delft, the Netherlands
Pim W. J. M. Willemsen, Vincent van Zelst, Vera M. van Bergeijk & Mark Klein Breteler
Royal Netherlands Institute for Sea Research (NIOZ), Yerseke, the Netherlands
Victoria G. Mason & Tjeerd J. Bouma
Utrecht University, Utrecht, the Netherlands
Victoria G. Mason & Tjeerd J. Bouma
Delft University of Technology, Delft, the Netherlands
Vincent van Zelst, Dimitrios Dermentzoglou, Akis Vouziouris & Alessandro Antonini
University of Twente, Enschede, the Netherlands
Jos R. M. Muller, Thomas J. van Veelen, S. Dzimballa, Kathelijne M. Wijnberg & Bas W. Borsje
Wetterskip Fryslân, Leeuwarden, the Netherlands
Paul Buring
Leibniz University Hannover, Hannover, Germany
Maike Paul
Authors
- Pim W. J. M. Willemsen
- Victoria G. Mason
- Vincent van Zelst
- Vera M. van Bergeijk
- Mark Klein Breteler
- Jos R. M. Muller
- Dimitrios Dermentzoglou
- Akis Vouziouris
- Thomas J. van Veelen
- S. Dzimballa
- Kathelijne M. Wijnberg
- Antonius J. F. Hoitink
- Paul Buring
- Maike Paul
- Alessandro Antonini
- Tjeerd J. Bouma
- Bas W. Borsje
Contributions
P.W.J.M., V.G.M., T.J.B. and B.W.B. conceptualized the work. P.W.J.M. and V.Z. performed the global analysis. PWJM, VGM, VMB, MKB, TAJFH, TJB and BWB prepared the visual materials and contributed to visualization. P.W.J.M. prepared the original draft. All authors except K.W. and T.A.J.F.H. performed experiments. All authors contributed to the methodology and review and editing of the manuscript.
Corresponding author
Correspondence to Pim W. J. M. Willemsen.
Ethics declarations
Competing interests
The authors declare no conflict of interest.
Peer review
Peer review information
Nature thanks Rusty Feagin, James Megonigal, and the other, anonymous, reviewer(s) for their contribution to the peer review of this work. Peer reviewer reports are available
Additional information
Publisher’s note Springer Nature remains neutral with regard to jurisdictional claims in published maps and institutional affiliations.
Extended data figures and tables
Extended Data Fig. 1 Global salt marsh vegetation comparison.
Vegetation above-ground biomass (a) and vegetation stem length (b) measurements before the storm season between late August and November (“BS (Before Storm)”) and after the storm season in March and April (“AS (After Storm)”). Elymus athericus is measured during our experiment (“Ely DF”) at the start in the field and flume and at the end in the flume. For verification Elymus athericus is compared with other studies quantifying Elymus spp. and salt marsh vegetation species with stems, including Spartina spp. and Phragmites spp. Numbers indicate references to the studies from which vegetation data are derived from6,19,71,72,73,74,75,76,77,78,79,80.
Extended Data Fig. 2 Storm events lead to decreasing wave attenuation due to vegetation damage (return period of 1,000 years).
Water depth at the seaward salt marsh edge, and distribution of water depths over all transects (a), exposure duration for progressive vegetation damage and distribution (b), relative stem height decrease and distribution (c) and GLM-predicted attenuation by vegetation and distribution per wave attenuation percentage class and incoming wave height bin (d) for a return period of 1,000 years.
Extended Data Fig. 3 Storm event leads to decreasing wave attenuation due to vegetation damage, model results with increased vegetation height (return period of 100 years).
Exposure duration for progressive vegetation damage and distribution (a), relative stem height decrease and distribution (b) and GLM-predicted attenuation by vegetation and distribution per wave attenuation percentage class and incoming wave height bin (c), calculated for a scenario where vegetation height is increased by 100%.
Extended Data Fig. 4 Storm event leads to decreasing wave attenuation due to vegetation damage, model results with increased vegetation height (return period of 1,000 years).
Exposure duration for progressive vegetation damage and distribution (a), relative stem height decrease and distribution (b) and GLM-predicted attenuation by vegetation and distribution per wave attenuation percentage class and incoming wave height bin (c), calculated for a scenario where vegetation height is increased by 100%.
Extended Data Fig. 5 Storm events lead to decreasing wave attenuation due to vegetation damage, model results with increased vegetation height and damage (return period of 100 years).
Exposure duration for progressive vegetation damage and distribution (a), relative stem height decrease and distribution (b) and GLM-predicted attenuation by vegetation and distribution per wave attenuation percentage class and incoming wave height bin (c), calculated for a scenario where vegetation height is increased by 100% and vegetation damage is also increased by 100%.
Extended Data Fig. 6 Storm events lead to decreasing wave attenuation due to vegetation damage, model results with increased vegetation height and damage (return period of 1,000 years).
Exposure duration for progressive vegetation damage and distribution (a), relative stem height decrease and distribution (b) and GLM-predicted attenuation by vegetation and distribution per wave attenuation percentage class and incoming wave height bin (c), calculated for a scenario where vegetation height is increased by 100% and vegetation damage is also increased by 100%.
Extended Data Fig. 7 Erosion resistance marsh substrate.
Bed elevation change of individual locations per measurement in time referred to exposure duration (grey lines) with mean values per measurement in time (blue dot), standard deviation (blue shading) and error bar (black bars).
Supplementary information
Supplementary information (download DOCX )
Supplementary Tables 1 and 2, and Figs. 1 and 2. Supplementary Table 1: Experimental program for the Delta Flume tests at Deltares (Delft, the Netherlands). Supplementary Table 2: Overview of statistical significance between measurements in between experimental runs for vegetation stem height and biomass. Supplementary Fig. 1: Water depth during a storm event for a return period of 100 years. Supplementary Fig. 2: Water depth during a storm event for a return period of 1,00 years
Peer Review File (download PDF )
Rights and permissions
Open Access This article is licensed under a Creative Commons Attribution-NonCommercial-NoDerivatives 4.0 International License, which permits any non-commercial use, sharing, distribution and reproduction in any medium or format, as long as you give appropriate credit to the original author(s) and the source, provide a link to the Creative Commons licence, and indicate if you modified the licensed material. You do not have permission under this licence to share adapted material derived from this article or parts of it. The images or other third party material in this article are included in the article’s Creative Commons licence, unless indicated otherwise in a credit line to the material. If material is not included in the article’s Creative Commons licence and your intended use is not permitted by statutory regulation or exceeds the permitted use, you will need to obtain permission directly from the copyright holder. To view a copy of this licence, visit http://creativecommons.org/licenses/by-nc-nd/4.0/.
About this article

Cite this article
Willemsen, P.W.J.M., Mason, V.G., Zelst, V.v. et al. The contribution of salt marshes to wave attenuation during extreme storms. Nature (2026). https://doi.org/10.1038/s41586-026-11145-8
Received:
Accepted:
Published:
Version of record:
DOI: https://doi.org/10.1038/s41586-026-11145-8